Gianluca GRENCI
Research Assistant Professor, Department of Biomedical Engineering, National University of Singapore
Facility Manager, Nano and Microfabrication Core
mbigg@nus.edu.sg
Level 10 T-Lab
National University of Singapore
5A Engineering Drive 1
Singapore 117411
Hu Yuqi
Research Assistant, Yu Group
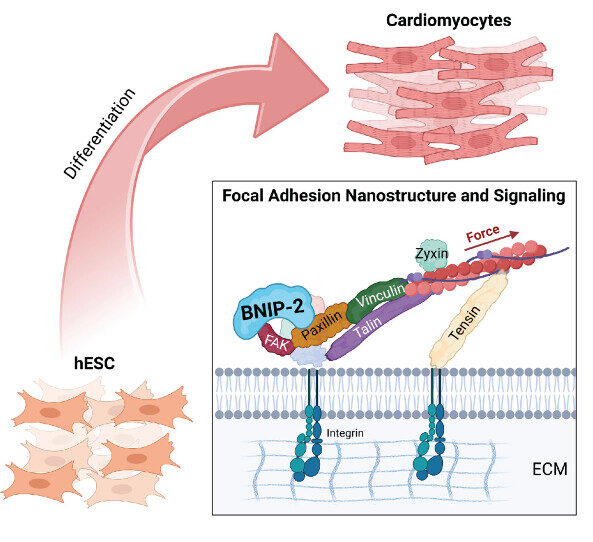
The Nano-Heartbuilder: BNIP-2 Influences Mechanosensing in Cardiomyoblast Differentiation
Researchers from the Low Lab at MBI discover a crucial role for the scaffold protein BNIP-2 in orchestrating focal adhesion dynamics during early heart development, offering new insights into heart regeneration strategies.
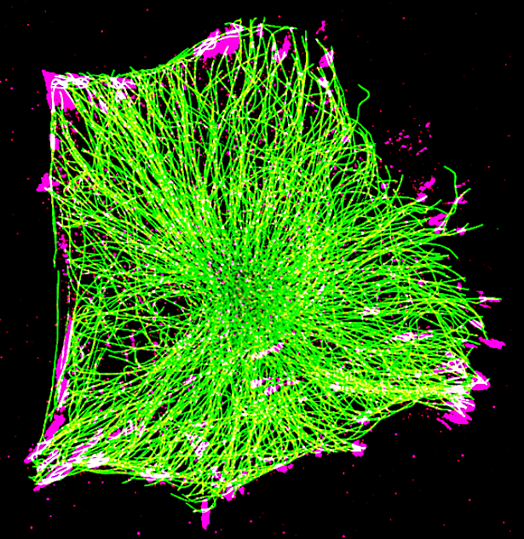
Shedding Light on Local Microtubule Regulation of Focal Adhesions
Researchers from the Bershadsky Lab at MBI utilized optogenetics to unlock the role of microtubules in regulating focal adhesion disassembly, an important step in cell migration. http://www.mbi.nus.edu.sg/featured-research/microtubules-and-cell-movement-a-closer-look-at-focal-adhesion-disassembly
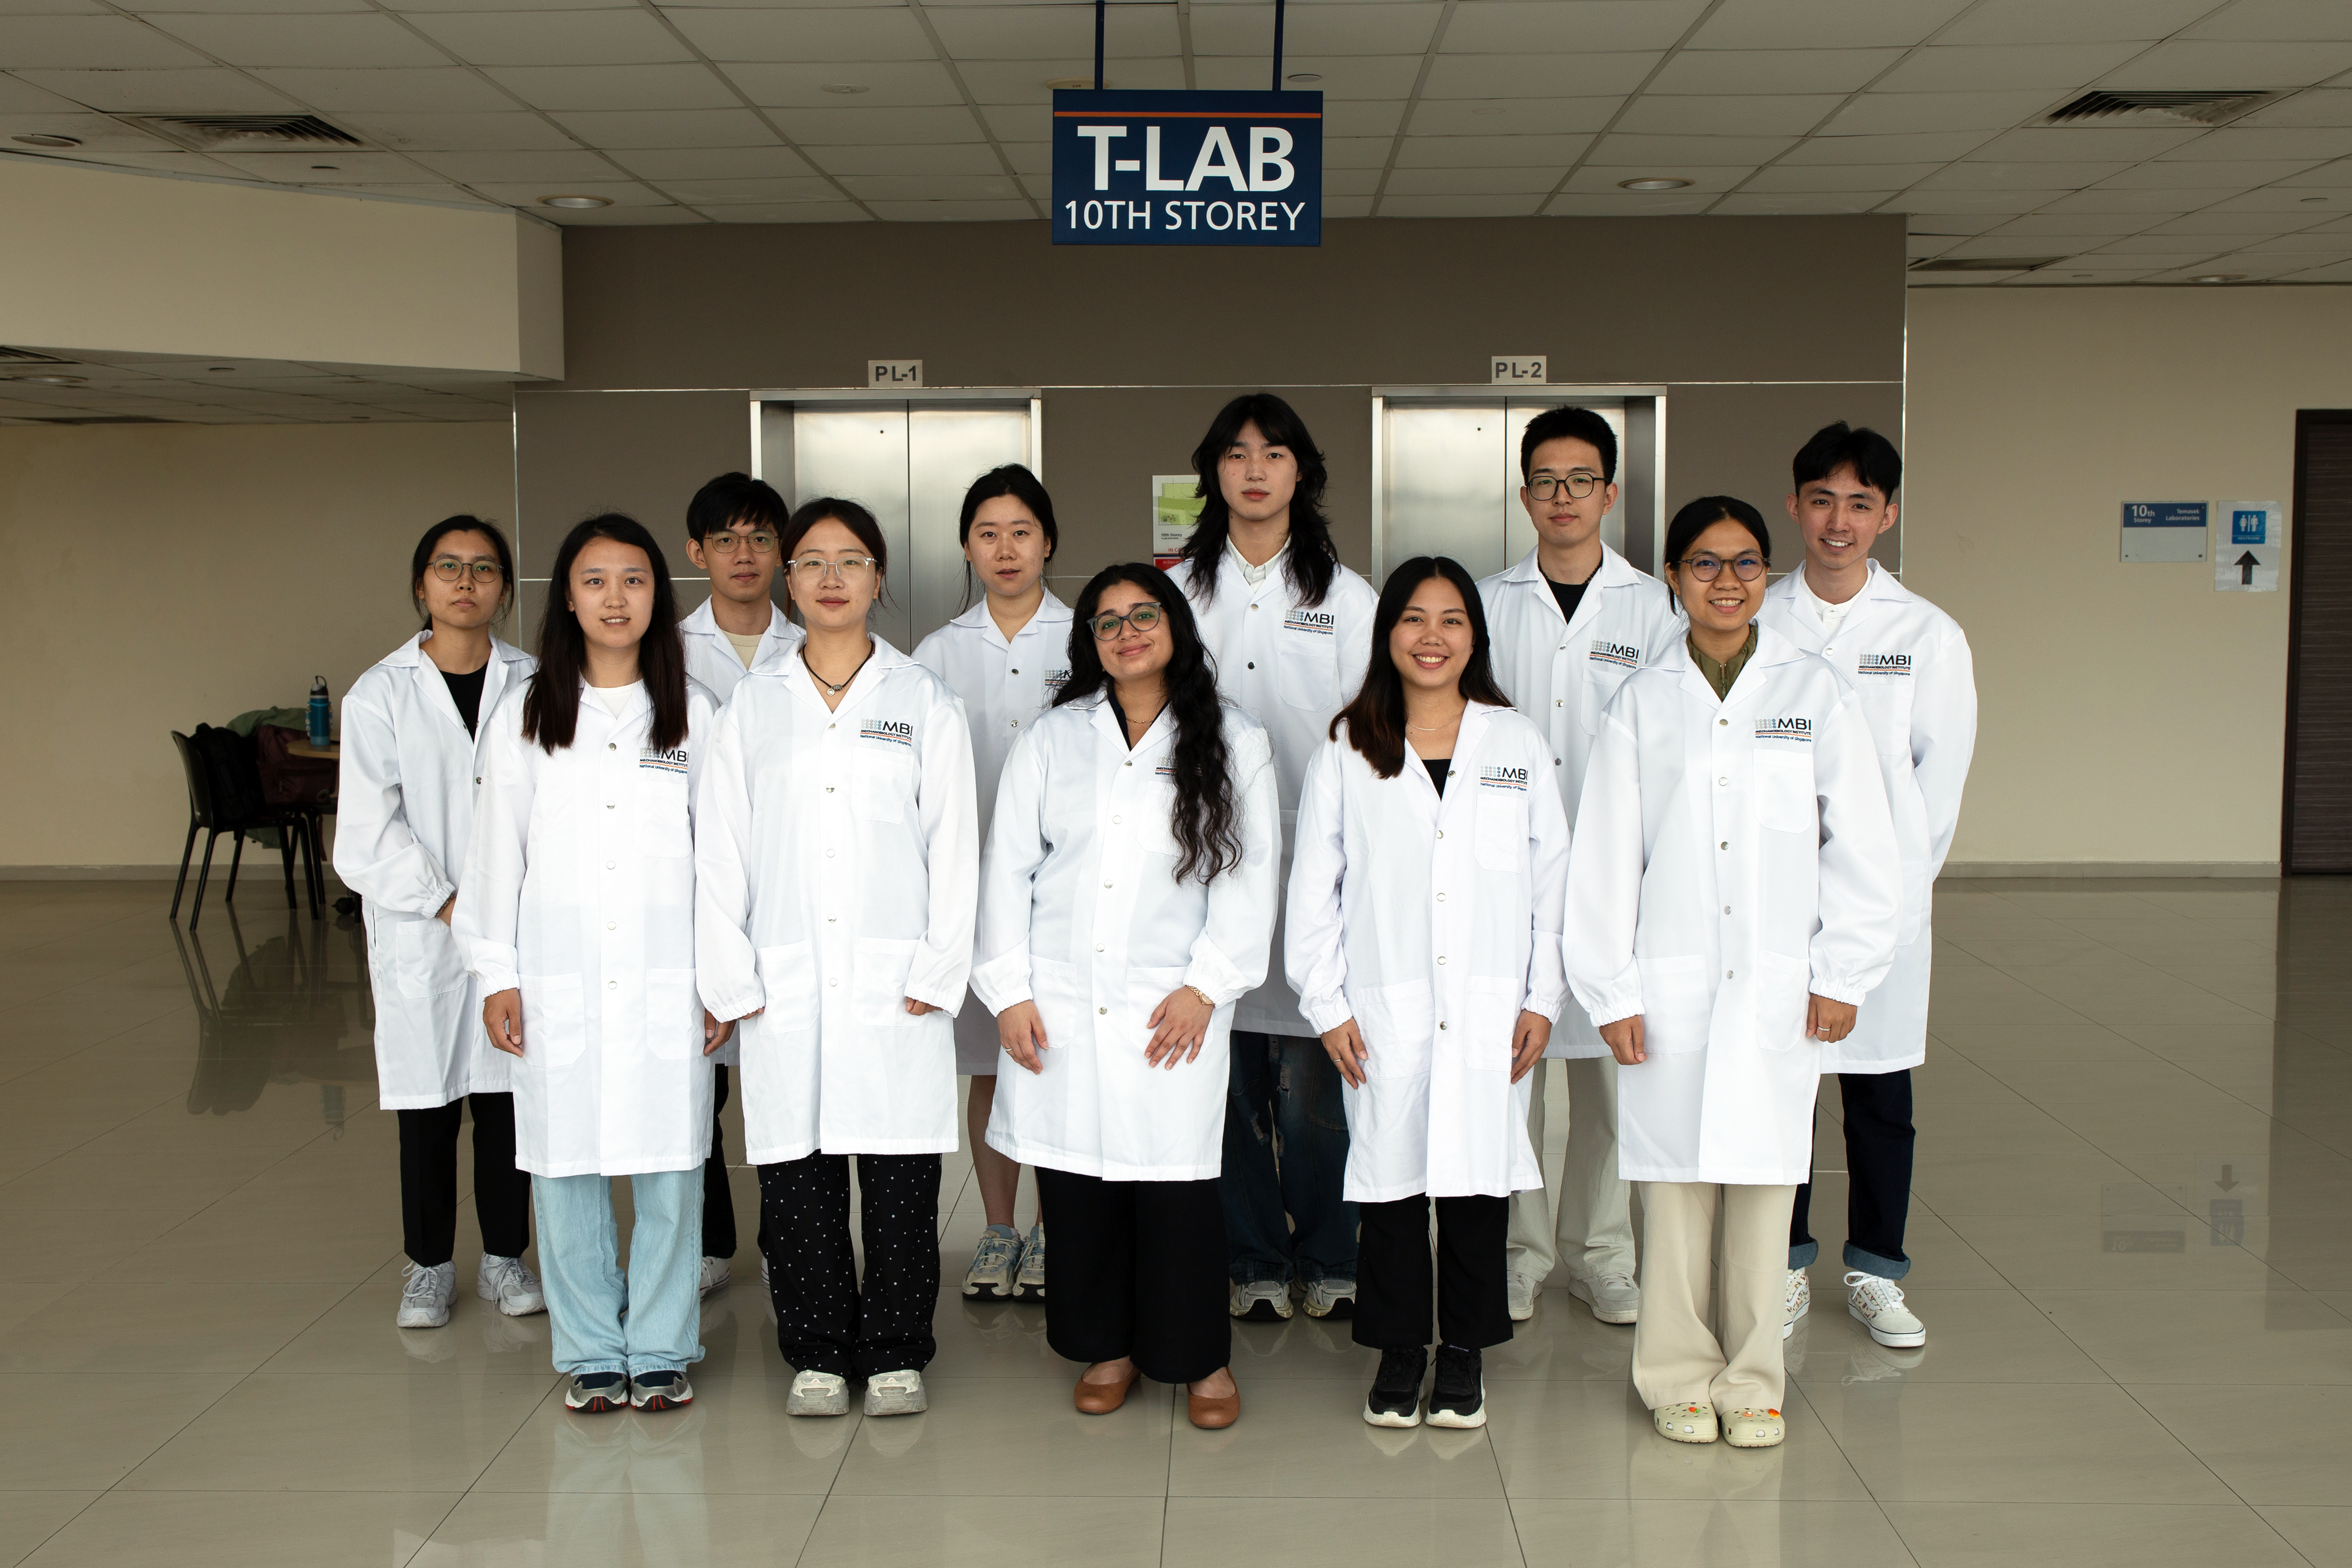
A Warm Welcome to the 2025 Ph.D Cohort!
MBI is delighted to welcome the 2025 cohort of Ph.D students. Coming from a rich tapestry of countries – China, Vietnam, Singapore, India and the Philippines – these eleven outstanding individuals bring with them interdisciplinary expertise and fresh perspectives that will enrich MBI’s vibrant research community.
Neha Paddillaya
Research Fellow, Chan Group
Privita Edwina
Research Fellow
Gianluca Grenci
Research Assistant Professor, Facility Manager
Research Interests
Microfluidics, Micro-optical systems for live cell imaging
Our laboratory is primarily interested in the application of micro/nano fabrication technology to biological science. We exploit standard and advanced micro-fabrication tools in order to design and produce systems and devices for cell culturing and imaging. Examples of such devices are: topographically and/or chemically micro-textured environments, microfluidic devices, micro-optical systems and more.
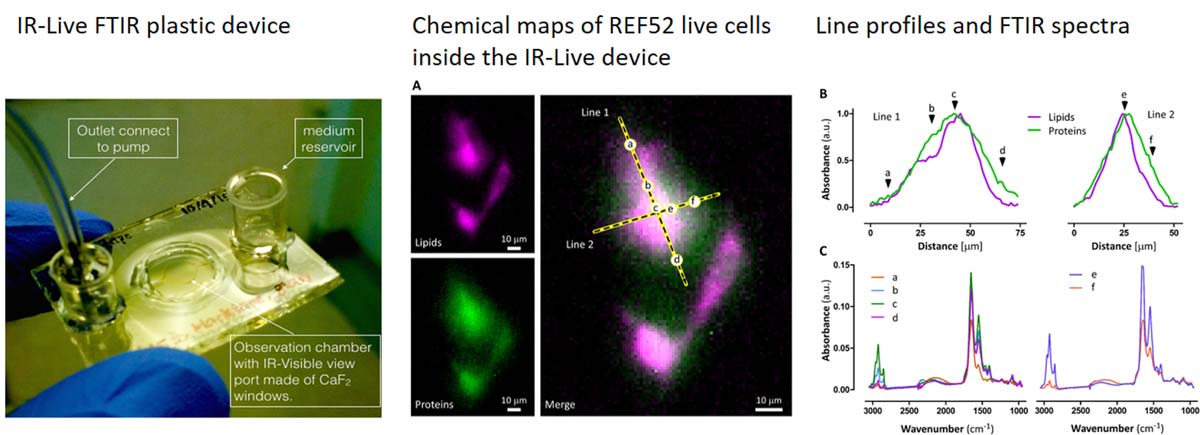
We are also interested in developing microfluidic devices for FTIR spectromicroscopy of living cells. FTIR is an imaging technique that is intrinsically label-free and requires minimal sample preparation; when coupled with microscopy and high brilliance IR sources it allows the acquisition of chemical maps at a resolution which is diffraction limited. Absorption of IR photons induces very low or no damage at all, therefore it is in principle possible to observe for prolonged time the behaviour of living cells. Our research activity is intended to develope microfludic platforms suitable for FTIR (key parameters are optical transparency and low IR absorption) while keeping cells alive and healthy; a beneficial feature provided by micro-fabrication approach is the possibility to control of the chemical environment at the micro-scale.
Research Areas
Micro/nano engineering, microfluidic, FTIR
Biography
Dr Gianluca Grenci joined MBI in 2012 as a research fellow and head of the Micro Fabrication Core facility. Previously he was employed at the LILIT micro/nano fabrication group (IOM-CNR, Trieste, IT) for a total of 6 years, during which he was mainly involved in the design and fabrication of microfluidic devices for synchrotron-light related spectroscopic techniques, such as SAXS and FTIR. He thus developed extensive practical knowledge on all the major lithographic technologies (UV and EB lithography, wet/dry etching, soft-lithography, thin films deposition), plus some less usual and/or more advanced technique, such as X-ray Lithography and LIGA.
He did his PhD in the field of applied superconductivity, in a project aimed to develop a current cryo-comparator (CCC) using high critical temperature superconductors of the cuprate family (YBCO) in the form of a thick film deposited onto a large area, complex shaped silver substrate.
Education
PhD Polytechnic of Torino, DISPEA
Recent Publications
- Zhang Z, Canela A, Kurisu J, Zou P, Kawaue T, Nakazawa N, Takeda N, Saeki M, Utsunomiya M, Bilgic M, Ishidate F, Grenci G, Furuta T, Kishi Y, Sasanuma H, and Kengaku M. Confined migration induces non-lethal DNA damage in developing neurons. Nature 2026;. [PMID: 42310452]
- Gandin A, Torresan V, Panciera T, Grenci G, Vanni G, Citron A, Marchionni M, Battilana G, Pelosin M, Busetto R, Piccolo S, and Brusatin G. Flexible high-resolution ECM micropatterning. Nat Protoc 2026;. [PMID: 42129485]
- Dunsing-Eichenauer V, Hummert J, Chardès C, Schönau T, Guignard L, Galland R, Grenci G, Tillmann M, Koberling F, Nock C, Sibarita J, Viasnoff V, Antolovic IM, Erdmann R, and Lenne P. Fast volumetric fluorescence lifetime imaging of multicellular systems using single-objective light-sheet microscopy. Commun Biol 2025;. [PMID: 41315677]
- Jiang X, Xu P, Feng F, Grenci G, and Saw TB. Revealing Electromechanical Control of Tissue Homeostasis Using a Two-Layer Microfluidic Device. J Vis Exp 2025;(223). [PMID: 41052031]
- Cabillic M, Forriere H, Bettarel L, Butler C, Neuhaus A, Idrissi I, Sambrano-Lopez ME, Rossbroich J, Müller L, Ries J, Grenci G, Viasnoff V, Levet F, Sibarita J, and Galland R. In-depth single molecule localization microscopy using adaptive optics and single objective light-sheet microscopy. Nat Commun 2025; 16(1):8362. [PMID: 40993142]
- Mu B, Rutkowski DM, Grenci G, Vavylonis D, and Zhang D. Ca2+-dependent vesicular and non-vesicular lipid transfer controls hypoosmotic plasma membrane expansion. BMC Biol 2025; 23(1):207. [PMID: 40629316]
- Ong HT, Karatas E, Poquillon T, Grenci G, Furlan A, Dilasser F, Mohamad Raffi SB, Blanc D, Drimaracci E, Mikec D, Galisot G, Johnson BA, Liu AZ, Thiel C, Ullrich O, , Racine V, and Beghin A. Digitalized organoids: integrated pipeline for high-speed 3D analysis of organoid structures using multilevel segmentation and cellular topology. Nat Methods 2025;. [PMID: 40369245]
- Arora A, Rizvi MS, Grenci G, Dilasser F, Fu C, Ganguly M, Vaishnavi S, Paramsivam K, Budnar S, Noordstra I, Yap AS, and Viasnoff V. Viscous dissipation in the rupture of cell-cell contacts. Nat Mater 2025;. [PMID: 40355570]
- Nakazawa N, Grenci G, Kameo Y, Takeda N, Sawada T, Kurisu J, Zhang Z, Toma K, Adachi T, Nonomura K, and Kengaku M. PIEZO1-dependent mode switch of neuronal migration in heterogeneous microenvironments in the developing brain. Cell Rep 2025; 44(3):115405. [PMID: 40053456]
- Suryana M, Produit T, Yang H, Birarda G, Shanmugar JV, Krivitsky L, Paterova A, and Grenci G. Infrared imaging with visible light in microfluidic devices: the water absorption barrier. Analyst 2024;. [PMID: 39692693]
Selected Publications
- Mona Suryana, Jegan V. Shanmugarajah, Sivakumar M. Maniam, Gianluca Grenci. Soft Lithographic Procedure for Producing Plastic Microfluidic Devices with View-ports Transparent to Visible and Infrared Light
- Mohammed Ashraf, Sree V. Sundararajan, Gianluca Grenci. Low-power, low-pressure reactive-ion etching process for silicon etching with vertical and smooth walls for mechanobiology application
Lab Members
What is actin nucleation?
What is actin nucleation? The first step in actin polymerization is known as ‘nucleation’. This step sees the formation of an actin nucleus, which is essentially a complex of three actin monomers, from which [...]
How does Arp2/3-mediate the nucleation of branched filaments?
How does Arp2/3-mediate the nucleation of branched filaments? The Arp2/3 complex is composed of 7 evolutionarily conserved subunits (Arp2, Arp3, ARPC1-C5) that are structurally similar to the barbed end of actin [1]. The complex [...]
How do actin filaments grow?
How do actin filaments grow? Actin Filaments (F-actin) grow from the polymerization of G-actin monomers Actin is a highly abundant (10-100 micromolar on average),~42 kDa structural protein found in all eukaryotic cells (except for [...]
What is the role of cortactin in actin polymerization?
What is the role of cortactin in actin polymerization? Cortactin is a class II nucleation promoting factor (NPF) that binds to actin filaments and influences their stability. Cortactin specifically stabilizes Arp2/3-mediated branch points along [...]
What is the role of formin in actin polymerization?
What is the role of formin in actin polymerization? Formins promote the elongation of pre-existing filaments by removing barbed end capping proteins and forming a sleeve around the actin subunits. Formins are also capable [...]
What is the steady state phase of actin polymerization?
What is the steady state phase of actin polymerization? In the steady state phase, the filament dynamics enter a state of equilibrium where monomer disassembly from the (-) end and polymerization at the (+) [...]
What factors influence actin filament length and treadmilling?
What factors influence actin filament length and treadmilling? Several factors influence actin filament length and treadmilling. ATP binding on G-actin and free ATP-G-actin concentration ATP-binding on actin subunits modulates the dynamics of filament assembly, [...]
What factors regulate actin filament polymerization?
What factors regulate actin filament polymerization? Nucleation Promoting Factors (NPFs) (e.g. WASP, Scar/WAVE) modulate actin filament nucleation by bringing together actin monomers and pre-existing actin filaments, for example, during filopodial initiation where they recruit [...]
Actin Crosslinking
Actin Crosslinking Crosslinking of actin filaments is a critical step in cell motility and is a fundamental process in filopodia protrusion and lamellipodia formation. Smaller cross-linking proteins that are more globular (e.g. fascin) [...]
What are microtubules?
What are microtubules? Microtubules are hollow cylinders [1] that are approximately 25nm in diameter [2] and vary in length from 200 nm to 25 μm. They are formed by the lateral association of between [...]
What are intermediate filaments?
What are intermediate filaments? Intermediate filaments are a primary component of the cytoskeleton, although they are not found in all eukaryotes, and are absent in fungi and plants [1]. These filaments, which extend throughout [...]
I-BAR and Other Proteins/Factors
I-BAR and Other Proteins/Factors Proteins containing I-BAR (inverted Bin/amphiphysin/Rvs i.e. IRSp53 Missing-in-metastasis homology Domain or IMD) cooperate with various components of actin filament assembly, to promote filopodia protrusion, via several mechanisms including the stimulation [...]
Former Lab Members
What is actin nucleation?
What is actin nucleation? The first step in actin polymerization is known as ‘nucleation’. This step sees the formation of an actin nucleus, which is essentially a complex of three actin monomers, from which [...]
How does Arp2/3-mediate the nucleation of branched filaments?
How does Arp2/3-mediate the nucleation of branched filaments? The Arp2/3 complex is composed of 7 evolutionarily conserved subunits (Arp2, Arp3, ARPC1-C5) that are structurally similar to the barbed end of actin [1]. The complex [...]
How do actin filaments grow?
How do actin filaments grow? Actin Filaments (F-actin) grow from the polymerization of G-actin monomers Actin is a highly abundant (10-100 micromolar on average),~42 kDa structural protein found in all eukaryotic cells (except for [...]
What is the role of cortactin in actin polymerization?
What is the role of cortactin in actin polymerization? Cortactin is a class II nucleation promoting factor (NPF) that binds to actin filaments and influences their stability. Cortactin specifically stabilizes Arp2/3-mediated branch points along [...]
What is the role of formin in actin polymerization?
What is the role of formin in actin polymerization? Formins promote the elongation of pre-existing filaments by removing barbed end capping proteins and forming a sleeve around the actin subunits. Formins are also capable [...]
What is the steady state phase of actin polymerization?
What is the steady state phase of actin polymerization? In the steady state phase, the filament dynamics enter a state of equilibrium where monomer disassembly from the (-) end and polymerization at the (+) [...]
What factors influence actin filament length and treadmilling?
What factors influence actin filament length and treadmilling? Several factors influence actin filament length and treadmilling. ATP binding on G-actin and free ATP-G-actin concentration ATP-binding on actin subunits modulates the dynamics of filament assembly, [...]
What factors regulate actin filament polymerization?
What factors regulate actin filament polymerization? Nucleation Promoting Factors (NPFs) (e.g. WASP, Scar/WAVE) modulate actin filament nucleation by bringing together actin monomers and pre-existing actin filaments, for example, during filopodial initiation where they recruit [...]
Actin Crosslinking
Actin Crosslinking Crosslinking of actin filaments is a critical step in cell motility and is a fundamental process in filopodia protrusion and lamellipodia formation. Smaller cross-linking proteins that are more globular (e.g. fascin) [...]
What are microtubules?
What are microtubules? Microtubules are hollow cylinders [1] that are approximately 25nm in diameter [2] and vary in length from 200 nm to 25 μm. They are formed by the lateral association of between [...]
What are intermediate filaments?
What are intermediate filaments? Intermediate filaments are a primary component of the cytoskeleton, although they are not found in all eukaryotes, and are absent in fungi and plants [1]. These filaments, which extend throughout [...]
I-BAR and Other Proteins/Factors
I-BAR and Other Proteins/Factors Proteins containing I-BAR (inverted Bin/amphiphysin/Rvs i.e. IRSp53 Missing-in-metastasis homology Domain or IMD) cooperate with various components of actin filament assembly, to promote filopodia protrusion, via several mechanisms including the stimulation [...]